Complete Hibiscus Plant (Hibiscus L.) Guides
Growing Guide
Problems & Diseases
Seasonal Care
Flowering Season
Introduction
Hibiscus L. is an accepted genus of Malvaceae comprising a diverse assemblage of annual and perennial herbs, subshrubs, shrubs, and trees. Its native range is principally tropical and subtropical, and its members are characterized collectively by variable leaves, showy flowers, a usually conspicuous staminal column, and capsular fruits.
Classification
- Plant Type
- Shrub
- Lifecycle
- Perennial
- Leaf Habit
- Evergreen
- Native Region
- Australia & Oceania, Central America, Indian Subcontinent, Northern South America, Southeast Asia
- Plant Family
- Malvaceae
Ecologically, the genus occupies a broad range of habitats rather than a single characteristic ecosystem, including rain forests, seasonally dry vegetation, riverbanks, open vegetation, and other tropical and subtropical environments. The combination of considerable morphological variation and broad habitat occupancy is therefore central to understanding Hibiscus at the genus level.
Several Hibiscus species have long histories of cultivation, particularly as ornamentals, while particular members have also been cultivated for fibre or other uses. Cultural and economic significance is consequently species-dependent rather than uniform across the genus. Conservation status likewise cannot be assigned as a single genus-wide category from species-level assessments. Recent taxonomic treatment has also transferred numerous taxa historically placed in Hibiscus to other genera, making nomenclatural scope important when older literature is consulted.
Quick Plant Information
| Field | Value |
|---|---|
| Accepted name | Hibiscus L. |
| Family | Malvaceae |
| Common name | Hibiscus |
| Life form | Annual or perennial herbs, subshrubs, shrubs, or trees |
| Native range | Tropics and subtropics |
| Conservation status | No single genus-wide conservation status; assessments are generally made at the species level |
| Uses category | Primarily ornamental; selected species are cultivated for fibre, food, beverages, traditional uses, and other documented purposes |
Classification and Taxonomy
| Rank | Taxon |
|---|---|
| Kingdom | Plantae |
| Phylum | Streptophyta |
| Class | Equisetopsida |
| Subclass | Magnoliidae |
| Order | Malvales |
| Family | Malvaceae |
| Genus | Hibiscus L. |
The requested profile concerns the genus Hibiscus, so a species-rank row is not applicable. The classification above follows the current Kew taxonomic backbone used for this profile.
Related Species of Significance
| Species | Relationship | Distinguishing note |
|---|---|---|
| Hibiscus syriacus L. | Accepted species within Hibiscus | A representative species useful for comparison within the genus; its species-level characteristics should not be generalized to Hibiscus as a whole. |
| Sabdariffa gossypiifolia (Mill.) M.M.Hanes & R.L.Barrett | Current accepted name for a taxon formerly treated as Hibiscus sabdariffa L. | Illustrates a nomenclatural boundary relevant to literature retrieval. Older literature may continue to use Hibiscus sabdariffa. |
| Sabdariffa cannabina (L.) M.M.Hanes & R.L.Barrett | Current accepted name for a taxon formerly treated as Hibiscus cannabinus L. | Illustrates another transfer from historical Hibiscus usage to the currently accepted genus Sabdariffa. |
Taxonomic Context
The principal identity issue for Hibiscus is circumscription. Hibiscus L. remains an accepted genus in the current Kew treatment, but its present circumscription differs from some historical treatments. In particular, several taxa formerly published or widely cited under Hibiscus are now placed in Sabdariffa.
This distinction is important when interpreting older literature. Publications using historical Hibiscus combinations may refer to taxa that are currently accepted under a different genus or combination. Literature retrieval should therefore include relevant synonyms and historical combinations where appropriate.
The genus has also been subdivided differently by different authors, and molecular studies have contributed to changes in the interpretation of relationships within the group. Consequently, genus-level statements should be interpreted in relation to the taxonomic circumscription and source used.
Cytogenetics
| Parameter | Value | Source |
|---|---|---|
| Chromosome number | No single genus-wide value established | — |
| Ploidy level | No single genus-wide value established | — |
| Genome size | No single genus-wide value established | — |
No single chromosome number, ploidy level, or genome-size value can be assigned to Hibiscus as a genus. Species-specific studies demonstrate cytogenetic diversity across the group, including variation in chromosome number and ploidy.
The absence markers above therefore indicate that a single genus-wide value is not established, rather than an absence of cytogenetic research. Species-specific chromosome counts, ploidy estimates, and genome-size measurements are available for individual members, but these values should not be presented as representative of the genus as a whole.
Scientific Stability and Nomenclature
Hibiscus L. remains an accepted genus in the current Kew treatment. The name was validly published by Linnaeus in Species Plantarum in 1753 and is a conserved name (nom. cons.). Hibiscus syriacus L. is recorded as the conserved type name associated with the genus.
Nomenclatural stability is nevertheless circumscription-dependent. The current recognition of Sabdariffa as a separate accepted genus, containing taxa historically treated under Hibiscus, means that older literature may require synonym and combination checking before it is mapped onto the current taxonomic framework.
Growth Habit and Architecture
Hibiscus L. is structurally diverse at genus level, ranging from annual or perennial herbs and subshrubs to shrubs and trees. The principal architectural gestalt is therefore variable rather than diagnostic through stature alone. Indumentum is commonly composed of stellate hairs, although simple hairs and nearly glabrous surfaces also occur.
| Field | Value |
|---|---|
| Life form | Annual or perennial herbs, subshrubs, shrubs, or trees |
| Mature height | Variable among species; no single genus-wide value established |
| Stem type | Herbaceous to woody, depending on species |
| Bark/surface texture | Variable; surfaces may be glabrous, pubescent, hispid, or otherwise hairy |
| Branching pattern | Variable among species |
| Root morphology overview | Species-variable; a single genus-wide architectural description is not established |
| Distinguishing architectural feature | Marked diversity in growth form combined with characteristic Hibiscus floral architecture |
The genus is correspondingly difficult to identify from vegetative architecture alone. Floral and fruit characters provide more consistent genus-level recognition than plant stature or branching pattern.
Stem
Stem structure varies substantially across Hibiscus, reflecting the breadth of growth forms represented in the genus. In woody members, stems may become substantially lignified, whereas annual or herbaceous species may retain comparatively delicate stems. Surface indumentum can be useful diagnostically when combined with leaves and reproductive structures.
| Field | Value |
|---|---|
| Stem type | Herbaceous or woody, species-dependent |
| Surface texture | Glabrous to pubescent, hispid, or stellate-hairy |
| Young/mature colour | Variable among species |
| Internode length | Variable; no genus-wide diagnostic value established |
| Thorn/spine/wing status | Not a consistent genus-wide character |
| Internal structure | Not documented at genus-wide level sufficiently for a single diagnostic description |
Recommended Products
Disclosure: As an Amazon Associate, PlantsInfo may earn from qualifying purchases.
🌱 Plant Care Essentials
The following tools can help with pruning, plant health, soil management, and fruit garden maintenance.

Neem Oil for Plant Care
Natural plant protection against aphids, whiteflies, mites, and other common garden pests.

Fungicide for Root Care
Helps suppress soil-borne fungal diseases and supports healthier root systems.

Spray Bottle for Plants
Ideal for applying foliar sprays, neem oil solutions, and liquid plant treatments.

Rubber Hand Gloves
Protects hands during pruning, planting, soil preparation, and garden maintenance.
Leaves
Leaves are one of the most variable vegetative features in Hibiscus. They are generally petiolate and simple, but their blades may range from entire to deeply lobed; margins may be entire, toothed, or otherwise variously modified. Stipules are usually present and commonly narrow. Leaf shape and margin variation can therefore be important for species-level recognition, but cannot be reduced to one genus-wide leaf form.
| Field | Value |
|---|---|
| Presence | Present |
| Leaf type | Simple; digitately compound leaves are reported in some taxonomic treatments |
| Arrangement | Variable; generally petiolate leaves |
| Blade form | Entire to deeply lobed; species-variable |
| Margin | Entire to variously toothed |
| Colour | Not documented as a uniform genus-wide diagnostic character |
| Special features | Stipules usually present; foliar nectaries occur in some species |
Flowers
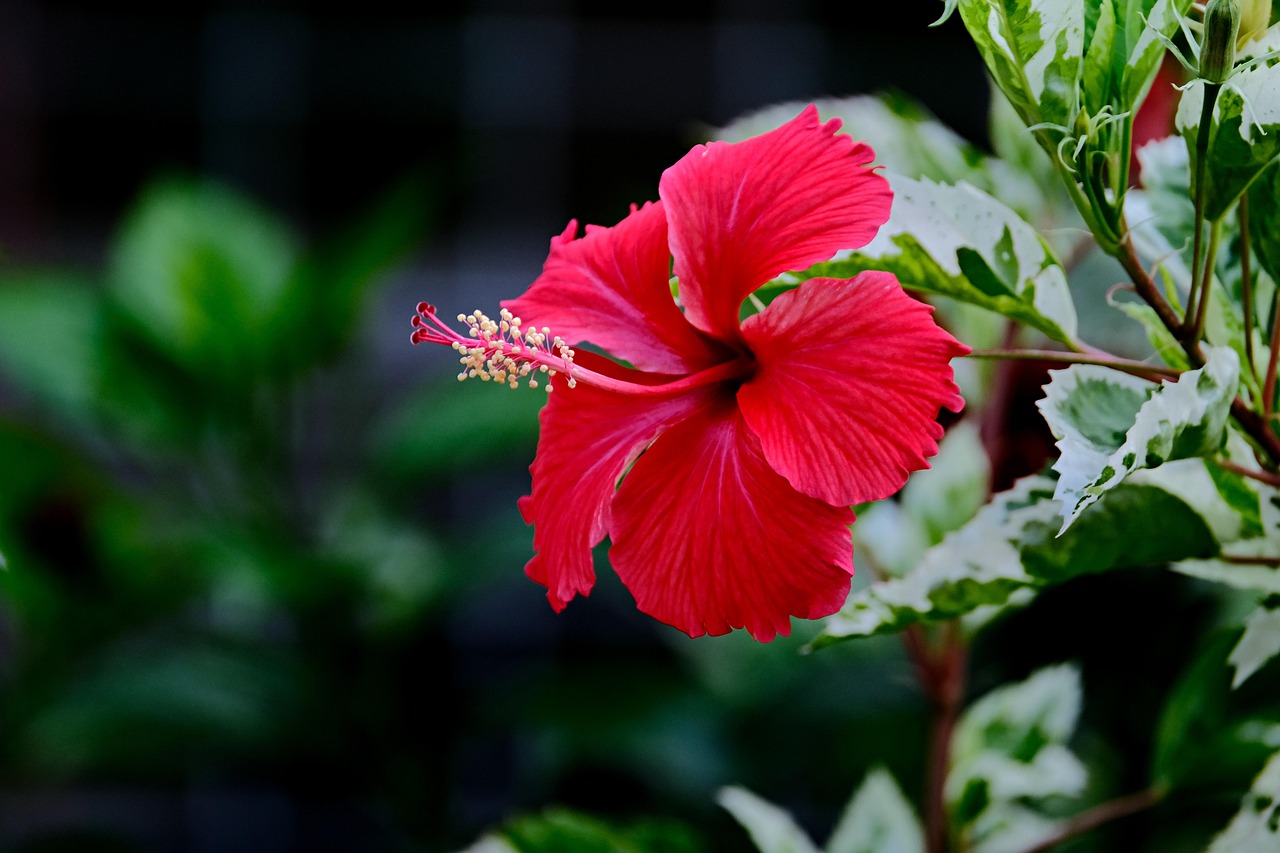
The flowers provide the strongest general morphological gestalt for recognizing Hibiscus: they are commonly conspicuous, five-merous, and associated with a prominent staminal column. Flowers are usually solitary in leaf axils, although reduction of upper leaves can produce terminal racemose or corymbose arrangements.
| Field | Value |
|---|---|
| Inflorescence type | Usually solitary and axillary; terminal arrangements also occur |
| Flower size | Variable among species |
| Sepals | Usually 5, forming a persistent 5-lobed calyx |
| Petals | Usually 5; commonly yellow, red, pink, purple, or white |
| Stamens | Numerous, associated with a staminal column |
| Pistil | Superior ovary, usually 5-locular; style commonly divided into 5 branches |
| Fragrance | Not a uniform genus-wide character |
| Anthesis | Variable among species |
The combination of showy five-merous flowers, an epicalyx that is commonly present, and a prominent staminal column is particularly useful for genus-level recognition. Floral size and colour, however, vary substantially among species.
Fruit
| Field | Value |
|---|---|
| Fruit type | Loculicidal capsule |
| Shape | Variable, including globose, ovoid, oblong, or angular forms |
| Surface features | Glabrous to hairy; some capsules are prominently angled or winged |
| Seed number | Usually several or more per locule |
The capsular fruit complements floral characters in field identification. Capsule architecture varies enough among species that individual fruit shapes should not be treated as universal Hibiscus characters.
Seeds
| Field | Value |
|---|---|
| Shape | Usually reniform |
| Surface | Glabrous to hairy; smooth to tuberculate |
| Number | Commonly several per locule |
Seed morphology is useful principally at species or species-group level because surface texture, pubescence, and dimensions vary considerably within the genus.
Root System
A sufficiently consistent genus-wide root architecture is not established in the available evidence. Root morphology is expected to vary with species and growth form, and the evidence available here does not support a single diagnostic rooting-depth or lateral-spread value.
Field Identification
At genus level, the most useful recognition combination is a showy five-merous flower with a conspicuous staminal column, usually accompanied by an epicalyx, followed by a capsular fruit. Vegetative characters alone are less reliable because leaf shape, growth form, indumentum, and stature are highly variable across the genus.
A particularly useful distinguishing feature is the combination of the staminal column and capsular fruit rather than any single leaf or stem character. Species-level identification requires more detailed characters and should be undertaken against an appropriate regional flora or taxonomic treatment.
Observed Morphological Variation
| Observation | Status | Notes |
|---|---|---|
| Substantial variation in leaf lobing and margin form | Normal variation | Leaf morphology varies substantially among Hibiscus species. |
| Hairy or nearly glabrous vegetative surfaces | Normal variation | Indumentum ranges from sparse or absent to conspicuous pubescence or hispidness among species. |
| Variation in flower colour | Normal variation | Yellow, red, pink, purple and white flowers are documented within the genus. |
| Herbaceous through woody growth forms | Normal variation | The genus includes herbs, subshrubs, shrubs and trees. |
Functional Traits
At the genus level, Hibiscus does not have a single experimentally established physiological strategy. The available evidence is strongly species- and cultivar-dependent. For example, drought-response experiments in H. mutabilis demonstrate stomatal regulation, osmotic adjustment, antioxidant defence, and changes in water-use efficiency, but those findings cannot be promoted to universal Hibiscus traits.
| Trait | Mechanism Description | Ecological Context |
|---|---|---|
| Stress-response plasticity | Species and cultivars can alter stomatal behaviour, osmotic regulation, antioxidant activity, and metabolite profiles under water deficit. | Demonstrated experimentally in H. mutabilis; not established as a uniform genus-wide response. |
| Photosynthetic response | Photosynthetic gas exchange can be constrained by both stomatal and biochemical processes under environmental stress. | Demonstrated in H. tiliaceus under salinity and aridity; the response should not be generalized to all Hibiscus. |
| Chemical defence / stress response | Phenolic and flavonoid metabolism changes under environmental stress in studied species. | Documented in individual species, including H. mutabilis; genus-wide physiological significance remains incompletely resolved. |
The evidence therefore supports physiological diversity and plasticity more strongly than a single shared functional syndrome. The distinction is important because the genus encompasses species occupying markedly different environments.
Physiological Integration
Species-specific evidence demonstrates that physiological traits can operate as an integrated response rather than independently. In drought-stressed H. mutabilis, greater water-use efficiency was associated with stronger stomatal regulation, osmotic adjustment, and antioxidant defence. However, a comparable integrated mechanism has not been established across Hibiscus as a whole.
No sufficiently comprehensive genus-wide synthesis was identified that would justify assigning one universal physiological trade-off or stress-response model to Hibiscus.
Phytochemistry
The genus has a substantial documented phenolic literature, but the chemical record is dominated by particular well-studied species and extracts rather than a uniform genus-wide metabolome. A genus-focused review identifies flavonoids, anthocyanins, and phenolic acids as recurring classes and reports repeated detection of several named compounds across the evaluated Hibiscus literature.
| Compound Class | Representative Compounds | Primary Location | Ecological or Biological Function |
|---|---|---|---|
| Flavonoids | Myricetin, quercetin, quercetin 3-glucoside, quercetin 3-rutinoside, myricetin 3-sambubioside | Species- and extract-dependent; organ-wide genus assignment not established | Documented phenolic constituents; biological functions have been investigated experimentally, but a uniform ecological function is not established at genus level. |
| Phenolic acids | Chlorogenic acid, caffeic acid, coumaroylquinic acid, protocatechuic acid, gallic acid, syringic acid | Species- and extract-dependent | Recurrently characterized constituents; genus-wide ecological function remains insufficiently established. |
| Anthocyanins | Delphinidin 3-sambubioside, cyanidin 3-sambubioside, cyanidin 3-glucoside | Particularly documented in pigmented tissues of studied species | Pigment chemistry is documented; specific ecological functions should not be generalized across the genus. |
The strongest genus-level chemical conclusion is therefore recurrence of phenolic chemistry, not chemical uniformity. The available literature also shows that extraction method can substantially influence the phenolic composition recovered from Hibiscus material, which complicates direct comparison among studies.
Phytochemical Organ Distribution
A single genus-wide organ-distribution map cannot be established. Direct organ-specific studies exist for individual species—for example, leaf chemistry has been characterized in H. sabdariffa, while petal chemistry has been characterized in H. rosa-sinensis—but these cannot be merged into a universal Hibiscus organ profile.
Phytochemical Significance
Phenolic compounds constitute the most extensively characterized chemical domain in the genus-level literature. Repeatedly identified compounds include myricetin and quercetin derivatives, chlorogenic and caffeic acids, protocatechuic and gallic acids, and anthocyanins such as delphinidin 3-sambubioside and cyanidin 3-sambubioside.
The characterization maturity is uneven. H. sabdariffa has received particularly intensive chemical investigation, including detailed characterization of anthocyanins, phenolic acids, and flavonoids, whereas other Hibiscus species remain much less comprehensively characterized.
The dominant organs are therefore species-dependent rather than demonstrably genus-wide. Calyces and leaves of H. sabdariffa and petals of H. rosa-sinensis are prominent research materials, but this distribution of research effort should not be interpreted as proof that those organs universally contain the highest concentrations of particular compounds across Hibiscus.
Specific synergistic or antagonistic relationships among Hibiscus phytochemicals cannot be established at the genus level from the evidence reviewed here. Reported biological effects of extracts containing multiple compounds do not, by themselves, demonstrate chemical synergy.
The clearest research-concentration bias is toward a relatively small number of intensively studied species, especially H. sabdariffa, with additional substantial work on H. rosa-sinensis. Consequently, genus-level phytochemical conclusions are disproportionately informed by these taxa rather than by an evenly sampled representation of Hibiscus.
Evidence Hierarchy for Medicinal Use
Hibiscus applies to this conditional section because several constituent species, particularly the taxon currently accepted as Sabdariffa gossypiifolia (historically Hibiscus sabdariffa L.), have documented traditional, nutritional, pharmacological, and clinical research. The evidence, however, is species- and preparation-specific and cannot be treated as evidence for the genus uniformly.
| Evidence Layer | Status | Notes |
|---|---|---|
| Traditional Use | Documented | Traditional medicinal use is well documented for Sabdariffa gossypiifolia (historically Hibiscus sabdariffa), including preparations of the calyces. This does not establish equivalent use across Hibiscus. |
| Nutritional Evidence | Documented | Food use and nutritional characterization are documented for species including Sabdariffa gossypiifolia (historically Hibiscus sabdariffa) and Hibiscus rosa-sinensis. |
| In Vitro Studies | Documented | Numerous in-vitro investigations exist, particularly for Sabdariffa gossypiifolia extracts and phenolic constituents. |
| Animal Studies | Documented | Animal studies have investigated physiological and pharmacological effects of Sabdariffa gossypiifolia and other species historically or currently associated with Hibiscus. |
| Human Clinical Studies | Documented | Randomized and other clinical studies exist for Sabdariffa gossypiifolia, particularly involving blood-pressure and metabolic outcomes. |
| Regulatory Recognition | No genus-wide recognition identified | No genus-wide therapeutic regulatory recognition was identified in the reviewed evidence. Regulatory status, where applicable, should be assessed for the specific species, preparation, indication, and jurisdiction. |
| Unsupported Commercial Claims | Partial | Commercial products containing Hibiscus, particularly products associated with Sabdariffa gossypiifolia (historically Hibiscus sabdariffa), make health-related claims. Published reviews identify the need for stronger clinical evidence and better characterization of preparations. |
The evidence hierarchy is therefore broad but taxonomically uneven. The best-developed medicinal evidence concerns Sabdariffa gossypiifolia (historically Hibiscus sabdariffa), rather than Hibiscus as an undifferentiated genus.
Evidence Assessment
Traditional-use evidence substantially exceeds genus-wide clinical evidence because medicinal practice and research have focused on particular species and preparations. For Sabdariffa gossypiifolia (historically Hibiscus sabdariffa), clinical studies have investigated antihypertensive and other physiological effects, while reviews report generally good tolerability in the preparations studied. However, the clinical literature remains heterogeneous and has limitations involving sample size, preparation standardization, and study design.
The strongest evidence category is therefore human clinical evidence for particular preparations of particular species, rather than evidence supporting medicinal efficacy of Hibiscus generally. The weakest category is genus-wide therapeutic inference: evidence from Sabdariffa gossypiifolia or Hibiscus rosa-sinensis cannot establish efficacy for other Hibiscus species.
Commercial health claims should consequently be interpreted at the species-and-preparation level. Published reviews explicitly call for larger, better-controlled clinical trials using phytochemically characterized preparations.
Nutritional Composition
Food use is documented for several Hibiscus species, so nutritional evidence is applicable. However, the available quantitative values are species-, organ-, preparation-, and moisture-basis-specific. They should therefore not be presented as genus-wide nutritional constants.
| Nutrient | Value per 100 g | Notes | Source |
|---|---|---|---|
| Protein | 26.32 g | Brown Sabdariffa gossypiifolia seeds (historically Hibiscus sabdariffa), dry-matter basis; value is species- and tissue-specific. | Getachew et al., 2020 |
| Fat | 15.58–18.00 g | Sabdariffa gossypiifolia seeds (historically Hibiscus sabdariffa), dry-matter basis; reported variation among seed samples. | Getachew et al., 2020 |
| Energy | 371.64–376.69 kcal | Sabdariffa gossypiifolia seeds (historically Hibiscus sabdariffa), dry-matter basis. | Getachew et al., 2020 |
| Iron | 15.71 mg | Fresh Sabdariffa gossypiifolia leaves (historically Hibiscus sabdariffa); species- and tissue-specific. | Isingoma et al., 2026 |
| β-Carotene | 9.30 mg | Fresh Sabdariffa gossypiifolia leaves (historically Hibiscus sabdariffa); species- and tissue-specific. | Isingoma et al., 2026 |
These values demonstrate nutritional characterization of individual edible Hibiscus-related materials rather than a representative genus-wide composition.
Nutritional Significance
The nutritional significance of Hibiscus is concentrated in particular edible species and plant organs. The taxon currently accepted as Sabdariffa gossypiifolia (historically Hibiscus sabdariffa) has been investigated as a food material using leaves, calyces and seeds. Its seeds have been reported to provide substantial protein, fat and energy on a dry-matter basis, while studies of leaves have reported measurable concentrations of minerals and provitamin A compounds.
Nutrient measurements can differ materially among plant organs, moisture conditions and processing states. Consequently, values obtained from fresh leaves should not be directly compared with dry-matter values from seeds without accounting for the analytical basis.
Bioavailability can also differ from total nutrient content. In Sabdariffa gossypiifolia calyces (historically Hibiscus sabdariffa), only a fraction of measured iron was extractable into a beverage, while polyphenol–iron interactions may further affect bioaccessibility. Processing therefore matters, and a high analytical mineral concentration should not automatically be interpreted as equivalent nutritional availability.
Documented ecotype or wild-versus-cultivated variation cannot be generalized to Hibiscus as a genus from the evidence reviewed here.
Soil Ecology and Mycorrhizal Associations
Soil-biological evidence is species-specific and comparatively limited at genus level. A rhizosphere microbiome study of H. sabdariffa investigated healthy and diseased plants and found that fungal and bacterial community composition varied with plant health and geographic plot. The fungal family Nectriaceae was more abundant in diseased rhizospheres, while bacterial community structure showed a stronger geographic component than disease-status component.
A bacterial isolate, Sphingomonas rhizophila, has also been described from the rhizosphere of H. syriacus. This establishes a documented rhizosphere association, but isolation or co-occurrence does not by itself demonstrate a beneficial functional interaction.
No sufficiently consistent genus-wide evidence was identified here to establish a characteristic mycorrhizal association, a defined rhizosphere bacterial consortium, or a genus-wide allelopathic mechanism. These subjects therefore remain species- and study-dependent.
Toxicity and Safety
| Subject | Toxic Compounds | Clinical Effects | Source |
|---|---|---|---|
| Humans | No genus-wide toxic compound has been established; species-specific toxicological evidence exists, particularly for Sabdariffa gossypiifolia (historically Hibiscus sabdariffa). | Clinical studies of preparations of S. gossypiifolia have generally reported good tolerability in the studied conditions, but these findings cannot be generalized to all Hibiscus species or preparations. | Ali et al., 2005; Montalvo-González et al., 2022; Isingoma et al., 2026 |
| Cats | No verified genus-wide toxicity data identified during the current audit. | Genus-wide clinical effects cannot be established. ASPCA lists Hibiscus syriacus as non-toxic to cats, but this finding is species-specific. | ASPCA; current literature audit |
| Dogs | No verified genus-wide toxicity data identified during the current audit. | Genus-wide clinical effects cannot be established. ASPCA lists Hibiscus syriacus as non-toxic to dogs, but this finding is species-specific. | ASPCA; current literature audit |
| Livestock | No verified genus-wide toxicity data identified during the current audit. | Species-specific feeding literature exists, including Hibiscus rosa-sinensis, but it does not establish a genus-wide safety classification. | Valdivié & Martínez, 2022; current literature audit |
The safety evidence therefore supports neither a genus-wide toxicity designation nor a genus-wide guarantee of safety. The best-developed human safety evidence in the reviewed material concerns Sabdariffa gossypiifolia (historically Hibiscus sabdariffa). Reviews describe relatively low toxicity in the studied preparations while also identifying the need for additional safety research at higher doses and with longer exposure.
For companion animals, the ASPCA specifically lists Hibiscus syriacus as non-toxic to cats and dogs. This finding should not be extrapolated to every species currently or historically placed in Hibiscus.
Toxicity Context
Dose, preparation, and exposure duration matter. For Sabdariffa gossypiifolia (historically Hibiscus sabdariffa), animal toxicology studies have generally indicated relatively low acute and subacute toxicity, but older reviews also describe potentially adverse effects at excessive or prolonged exposure in experimental animals. Human clinical studies have generally reported good tolerability under the conditions studied; however, this evidence does not establish safety for every Hibiscus species, extract, concentration, or exposure duration.
Drug-interaction considerations have been discussed for S. gossypiifolia herbal products, particularly because some preparations may influence cardiovascular or renal physiological parameters. These considerations remain preparation-, dose- and patient-dependent rather than genus-wide.
No adequately established genus-wide conclusion concerning pregnancy-specific safety, renal vulnerability or hepatic vulnerability was identified in the reviewed evidence.
This profile does not constitute medical or veterinary advice.
Biogeographic Context
Hibiscus is a highly heterogeneous tropical and subtropical genus whose distribution spans multiple climatic and habitat settings rather than a single ecological envelope. Current Kew treatment describes the genus as occurring throughout the tropics and subtropics, with a smaller number of temperate species. The geographic pattern therefore reflects diversification across seasonally dry, humid, coastal, riparian, open, and forest-associated environments rather than one shared habitat specialization.
Dispersal history can also contribute substantially to distribution in particular lineages. In Hibiscus tiliaceus, for example, buoyant seeds and ocean-current dispersal are associated with its exceptionally broad pantropical coastal distribution, although the relative contribution of natural dispersal and historical human movement remains unresolved. Research is unevenly distributed among species: economically important taxa such as H. sabdariffa, H. cannabinus, H. rosa-sinensis, and H. tiliaceus are much better represented in ecological and cultivation literature than many wild congeners.
Habitat loss and collection pressure cannot be generalized across the genus from the available evidence. Conservation concerns are documented for individual taxa, but a genus-wide pressure assessment is not presently defensible.
Native Range and Distribution
The genus-level native range is best represented by documented regional occurrences rather than by assigning every locality recorded for individual species to the genus as a whole.
| Region | Countries or Sub-regions | Notes |
|---|---|---|
| Tropical Africa | West, Central, East and southern African regions | Multiple native species are documented, including species occupying seasonally dry tropical habitats. |
| Indian Subcontinent | India, Pakistan, Bangladesh, Sri Lanka | Native species occur across tropical and seasonally dry environments; individual species have narrower ranges. |
| Southeast Asia | Myanmar, Thailand and the Malay region | Native representatives occur across tropical and subtropical habitats. |
| Southern China and Taiwan | Southern and southeastern China; Taiwan | Includes species with tropical/subtropical as well as temperate ecological affinities. |
| Pacific Islands and Australasia | New Guinea and numerous Pacific island regions | New Guinea has six documented native species; Pacific distributions include both native and historically introduced lineages. |
| Tropical Americas | Mexico, Central America, Caribbean and parts of northern South America | Native representatives occur in tropical and subtropical environments, but individual species ranges vary substantially. |
The distribution should therefore be read as a genus-level synthesis of documented native regional occurrence, not as evidence that every Hibiscus species occurs throughout all listed regions.
Global Cultivation and Naturalisation
Cultivation is extensive but strongly concentrated in a subset of species. Ornamental cultivation is globally widespread, while food and fibre production is concentrated principally in particular species and cultivar groups.
| Region | Countries or Areas | Cultivation Status | Notes |
|---|---|---|---|
| South and Southeast Asia | India, Bangladesh, Thailand, Indonesia and neighbouring regions | Commercially established | H. sabdariffa is cultivated for food, beverages and fibre; other Hibiscus species are widely ornamental. |
| Tropical Africa | Sudan, Nigeria and other African production regions | Commercially established | H. sabdariffa has established food and fibre uses. |
| China and East Asia | China and surrounding regions | Commercially established | Ornamental cultivation is extensive; selected species are also cultivated for food or other uses. |
| Tropical and subtropical Americas | Mexico, Caribbean, Central America and parts of South America | Commercially established | Ornamental cultivation is widespread; roselle production occurs in selected areas. |
| Temperate regions | Europe, North America and comparable climates | Emerging / Experimental for tender taxa; established for hardy species | Cultivation success depends strongly on species; frost-sensitive tropical taxa have narrower outdoor envelopes. |
Cultivation Range Note: The strongest production evidence concerns H. sabdariffa, while ornamental cultivation encompasses a much broader group of species and hybrids. Literature is therefore heavily biased toward economically important taxa rather than representing the genus evenly. Cultivation outside native regions should not be interpreted automatically as naturalisation.
Natural Habitat
Hibiscus occupies a broad range of natural settings. Documented habitats include lowland tropical forest, secondary and open vegetation, seasonally dry tropical communities, riverbanks, coastal vegetation, strand and mangrove-associated habitats, and disturbed environments. New Guinea records particularly illustrate this ecological breadth, with species occurring from lowland rainforest through open vegetation with pronounced dry seasons to moist riverbanks.
Elevation is similarly heterogeneous. Individual species can be restricted to lowlands, while others extend into upland or montane environments. For example, H. tiliaceus is principally coastal but can occur inland and at higher elevations, whereas other species are associated with seasonally dry or even desert/shrubland environments.
Soil associations are likewise species-dependent. H. sabdariffa is documented from a broad range of soils when adequate drainage is available, whereas coastal taxa such as H. tiliaceus occupy substrates influenced by salinity and periodic marine inundation. No single genus-wide soil specialization is supported.
Disturbance response varies among species. Some Hibiscus occur naturally in open or disturbed habitats, while others are associated more strongly with forest, wetland, or coastal vegetation. The genus should consequently be regarded as ecologically heterogeneous rather than habitat-specialized.
Ecological Role
Evidence is moderate and strongly species-biased. The clearest documented roles concern floral resources, pollination, seed dispersal, and habitat-associated ecological functions.
| Role Type | Species or Agent Involved | Notes |
|---|---|---|
| Floral resource / pollination | Bees and other insects; Hibiscus spp. | Large flowers provide pollen and/or nectar resources. Species-specific studies document insect-mediated pollination. |
| Specialist pollination relationship | Ptilothrix bombiformis and H. moscheutos | The bee is a documented major pollinator of H. moscheutos in studied North American populations. |
| Generalist insect pollination | Bees and other insects; H. tiliaceus | Studies document insect-mediated pollination, including bees; the exact assemblage varies geographically. |
| Seed dispersal | Water; H. tiliaceus | Buoyant seeds and ocean-current dispersal contribute to long-distance distribution in this coastal species. |
| Habitat-associated plant resource | Coastal fauna; H. tiliaceus | The species forms part of coastal plant communities and provides documented fauna-associated resources, including butterfly larval-host relationships in Singapore. |
No genus-wide keystone or indicator status is established. The ecological importance of Hibiscus is better understood as species- and habitat-dependent, with particularly strong evidence for pollination and dispersal roles in selected taxa.
Invasive Status
Naturalisation outside native ranges is documented for members of the genus, but invasive impact is not a genus-wide characteristic.
| Region | Status | Impact | Management |
|---|---|---|---|
| New Guinea | Naturalised | Genus-level ecological impact not established from the available source | No genus-wide management response documented. |
| North America and other introduced regions | Naturalisation documented for particular species, including H. trionum and H. syriacus in some areas | Species-specific weed or invasive classifications occur, but these cannot be generalized to Hibiscus as a whole | Management is jurisdiction- and species-specific. |
Naturalisation therefore demonstrates establishment outside a native range but does not by itself establish invasive ecological impact. Species-level classifications should remain attached to the relevant species.
Optimal Climate Parameters
A defensible genus-wide numerical climate envelope cannot be established. The genus contains species occupying tropical, subtropical, seasonally dry, coastal, and temperate environments. The numerical evidence below is therefore retained as species-level environmental envelopes, principally from cultivated or ecologically characterized taxa, rather than converted into artificial genus-wide limits.
| Parameter | Optimal Range | Tolerance Range | Notes |
|---|---|---|---|
| Mean Annual Temperature | Not established for Hibiscus as a genus | Not established for the genus | Available quantitative evidence is predominantly species-specific and often expressed as growing-season or mean-monthly temperature rather than annual temperature. |
| Annual Rainfall | 800–1600 mm documented for H. sabdariffa cultivation | 900–2500 mm documented for H. tiliaceus habitat | These are species-specific envelopes and are not interchangeable with a genus-wide optimum or tolerance. |
| Day Temperature | 25–30°C mean monthly growing-season temperature for H. sabdariffa | 10–36°C reported growth range for H. sabdariffa | Species-specific cultivation evidence; not a genus-wide physiological threshold. |
| Humidity | >70% during the growing period of H. sabdariffa | Not established for the genus | High humidity requirement is documented for roselle production, not for all Hibiscus. |
| Dry Season | A drier period supports flowering and seed production in H. sabdariffa | Not quantified at genus level | Seasonal drying is important for some cultivated taxa but is not universal across the genus. |
The corresponding imperial temperature values are approximately 77–86°F for the documented H. sabdariffa growing-season mean-monthly optimum and 50–97°F for its reported growth range. Rainfall values of 800–1600 mm correspond to approximately 31.5–63.0 in, while 900–2500 mm corresponds to approximately 35.4–98.4 in annually.
The absence of a genus-wide mean annual temperature and tolerance range is a genuine evidence gap rather than a basis for constructing a synthetic range.
Climate Interpretation
The principal climatic limitation differs among Hibiscus lineages. Tropical cultivated taxa such as H. sabdariffa are constrained principally by frost and by the interaction between rainfall distribution and reproductive seasonality. A defined dry period can be advantageous for flowering and calyx/seed production, whereas excessive moisture can impair some production outcomes.
Coastal H. tiliaceus demonstrates a different climatic envelope, including environments with substantial annual rainfall and saline exposure. Conversely, temperate Hibiscus species demonstrate that the genus as a whole cannot be characterized as uniformly frost-sensitive.
The distinction between native occurrence and cultivation performance is important. Cultivation evidence is concentrated in economically important species and therefore does not establish the climatic limits of the remaining genus. Expansion into climates outside a particular species’ documented envelope cannot be inferred from the broader tropical/subtropical distribution of Hibiscus.
Stress Tolerance Profile
Only stress responses supported by species-specific physiological evidence are included.
| Stress Type | Tolerance Level | Physiological Response | Notes |
|---|---|---|---|
| Drought / water deficit | Supported | In H. mutabilis, drought-tolerant material maintained higher water-use efficiency through stronger antioxidant activity, osmotic regulation and stomatal regulation. | Demonstrated in particular cultivars; does not establish genus-wide drought tolerance. |
| Salinity | Verified | In H. tiliaceus, salinity altered stomatal conductance, photosynthetic activity and water-use efficiency; coastal populations showed greater physiological tolerance than an upland population in experimental comparisons. | Strong species- and population-specific evidence. |
| Salinity / ionic stress | Supported | Comparative work in H. tiliaceus identified population differences in K⁺/Na⁺ regulation and salt-responsive physiological and transcriptional responses. | Ecological differentiation among populations limits genus-wide extrapolation. |
Broad statements that Hibiscus is “hardy,” “drought tolerant,” or “salt tolerant” are therefore insufficient without specifying the species, population, and experimental context.
Compound Stress Assessment
No adequate genus-level evidence was identified for combined drought–heat, drought–salinity, heat–salinity, or other multi-stressor physiological responses.
The available studies generally isolate individual stresses, with the strongest examples concerning drought in H. mutabilis and salinity in H. tiliaceus. Consequently, interactions among stress-response pathways should remain a knowledge gap rather than being inferred from single-stress experiments.
Structural and Physiological Adaptations
At the genus level, adaptive interpretation is necessarily species-specific. The following traits have documented ecological significance beyond ordinary morphology.
| Adaptation | Mechanism Description | Ecological Context |
|---|---|---|
| Buoyant, water-dispersed seeds in hydrochorous species | Air space associated with a thick, water-impermeable seed coat allows seeds to remain afloat after release. | Documented in H. tiliaceus and H. moscheutos; supports dispersal along coastal, riverine, and wetland systems. (The Ecological Society of Japan) |
| Persistent underground caudex in H. moscheutos | A perennial underground stem/rootstock survives seasonal above-ground turnover and produces new flowering shoots. | Supports persistence in seasonally inundated and temperate wetland habitats. (US Forest Service R&D) |
| Fragmentation-assisted regeneration in H. moscheutos | Perennial clumps can fragment, with detached material transported by wind or water. | Provides a documented secondary regeneration and colonisation pathway in wetland populations. (Canada) |
| Coastal dispersal morphology in H. tiliaceus | Fruit and seed characteristics facilitate prolonged flotation and long-distance hydrochory. | Consistent with the species’ pantropical coastal distribution; the adaptive significance is strongly habitat-specific. (US Forest Service R&D) |
These examples should not be generalized to all Hibiscus. In particular, the presence of buoyant seeds or perennial caudices is not a genus-wide character.
Climate Change Vulnerability
| Factor | Assessment | Notes |
|---|---|---|
| Primary Climate Sensitivity Factors | Species-specific; precipitation and temperature are documented determinants | Climate-envelope modelling of Hibiscus mutabilis identified precipitation of the driest month as the strongest limiting variable, with annual precipitation, mean temperature, and temperature range also important. A separate Hibiscus syriacus model likewise identified precipitation and temperature as major determinants. These results represent species-level evidence and should not be generalized to the genus. |
| Key Threatening Climate Processes | Altered precipitation regimes, drought episodes, temperature shifts, and changing seasonal conditions | Documented modelling indicates that future suitability can change spatially within species. These results cannot be converted into a single genus-wide vulnerability trajectory. |
| Resilience Factors | Broad ecological and climatic diversity; species- and population-level physiological variation | The genus occupies diverse environments, but the relative contribution of individual resilience mechanisms varies among species and populations. |
| Confidence Level | Moderate for selected species; low for genus-wide projection | Published climate models exist for Hibiscus mutabilis and Hibiscus syriacus, but equivalent evidence is not available across the genus. No genus-wide climate-vulnerability model was identified. |
Phenological Calendar
Because Hibiscus includes annual herbs, perennial herbs, shrubs, and trees across contrasting climates, a single genus-wide calendar would be misleading. The table therefore preserves documented species-level examples and explicitly marks parameters that cannot be generalized.
| Event | Native Range Timing | Cultivated Range Timing | Environmental Triggers |
|---|---|---|---|
| Vegetative Growth Onset | Hibiscus moscheutos: spring emergence in Maryland, approximately April | Species-dependent; no genus-wide cultivated timing established | Seasonal temperature and moisture conditions are implicated for H. moscheutos, but a quantitative trigger was not established in the reviewed evidence. |
| Flower Bud Initiation | Species-specific; not established genus-wide | The taxon currently accepted as Sabdariffa gossypiifolia (historically Hibiscus sabdariffa) is documented as photoperiod-sensitive | A short-day response is documented for S. gossypiifolia; an exact critical photoperiod threshold was not established here. |
| Anthesis or Peak Flowering | Hibiscus moscheutos: late July–September in Maryland; peak around the second week of August | Strongly species- and latitude-dependent; no genus-wide cultivated period established | Geographic and seasonal conditions influence timing; no common genus-wide flowering trigger is established. |
| Fruit Development | Hibiscus moscheutos: approximately 3–4 weeks from flowering to fruit maturation | Species-specific | Timing is documented for H. moscheutos; a genus-wide developmental trigger is not established. |
| Fruit Maturation | Hibiscus moscheutos: late summer to autumn; mature capsules persist after flowering | Species-dependent | Seasonal reproductive progression is documented, but no genus-wide temperature or photoperiod threshold is established. |
| Seed Dispersal | Hibiscus moscheutos: principally autumn; most seeds released October–November in Chesapeake Bay studies | Species-dependent | Capsule dehiscence controls release in the documented example; water can subsequently transport buoyant seeds. |
| Dormancy or Rest Period | Perennial species may undergo seasonal above-ground dormancy; seed dormancy is documented in wetland Hibiscus | Annual species such as Sabdariffa gossypiifolia (historically Hibiscus sabdariffa) do not share the same perennial rest cycle | Hibiscus moscheutos has a seasonal perennial cycle, and its seeds possess physical dormancy. No single genus-wide dormancy pattern exists. |
Phenological Notes
Phenology is highly plastic across the genus. The strongest evidence for environmental control in the reviewed material concerns the taxon currently accepted as Sabdariffa gossypiifolia (historically Hibiscus sabdariffa), where flowering is associated with photoperiod, and Hibiscus moscheutos, where flowering and seed release vary with geographic location.
The available evidence therefore supports species- and latitude-dependent phenological schedules, rather than a common Hibiscus calendar.
Pollination Ecology
Hibiscus flowers commonly present a conspicuous reproductive structure in which the staminal column and stigmatic branches are accessible to floral visitors. This creates opportunities for insect-mediated pollen transfer, but pollination systems differ substantially among species. Documented systems include bee-mediated pollination, mixed selfing and outcrossing, and, in Hibiscus tiliaceus, both insect- and wind-associated pollen transfer.
| Parameter | Value | Notes |
|---|---|---|
| Primary Pollinators | Ptilothrix bombiformis and bumblebees in Hibiscus moscheutos | P. bombiformis accounts for much of the documented pollination in studied Maryland populations. |
| Secondary Pollinators | Other bees; moths, butterflies and flies may visit | Flower visitation does not necessarily establish effective pollination; effectiveness is best demonstrated for particular bee taxa in studied species. |
| Pollination Syndrome | Predominantly bee-associated in documented species; ambophily documented in Hibiscus tiliaceus | H. tiliaceus has documented melittophily and functional anemophily; pollination syndromes vary among species. |
| Floral Mechanism | Reproductive structures provide a landing and foraging surface and position pollen and stigmas for contact with visiting bees | In H. moscheutos, upturned style branches and flattened stigmas form an accessible landing surface; bee movement across anthers facilitates pollen transfer. |
| Reproductive System | Self-compatible in Hibiscus moscheutos and H. tiliaceus; mixed selfed and outcrossed seed production documented in H. moscheutos | Reproductive systems vary among species; self-compatibility should not be treated as universal for the genus. |
| Seed Dispersal Agent | Water documented for H. moscheutos and H. tiliaceus | Water dispersal is particularly important in coastal and wetland taxa; other species may use different mechanisms. |
| Reproductive Evidence Status | Partial to verified at species level | Effective pollination and breeding-system evidence is strong for selected species but uneven across the genus. |
| Human Intervention | Biologically feasible in selected species | Controlled crosses have produced cultivated Hibiscus hybrids, including crosses involving H. moscheutos. This establishes biological feasibility without implying a genus-wide compatibility pattern. |
Pollination Context
Self-compatibility and outcrossing coexist within the genus. In Hibiscus moscheutos, spatial separation of anthers and stigmas reduces the likelihood of within-flower selfing while between-flower selfing remains possible. Pollen-tube competition can also affect male reproductive success, and the timing of successive pollen deposition has been experimentally shown to influence paternity.
The evidence does not justify assigning a single pollination dependency or pollinator-decline vulnerability to Hibiscus as a genus. Such assessments require species- and population-specific reproductive data.
Vegetative Reproduction
| Parameter | Value | Notes |
|---|---|---|
| Vegetative Regeneration Capacity | Documented in selected perennial species | H. moscheutos regenerates repeatedly from established underground structures; H. tiliaceus can also regenerate vegetatively. (US Forest Service R&D) |
| Primary Regeneration Mechanism | Caudex sprouting; rhizomatous or stem-sprouting regeneration in selected taxa | H. moscheutos sprouts from the caudex, with rhizomatous regeneration reported in some populations; H. tiliaceus can regenerate from prostrate stems. (US Forest Service R&D) |
| Minimum Propagule Size | Not established | No defensible genus-wide minimum viable propagule size was identified. |
| Ecological or Invasive Significance | Conditional | Vegetative persistence can support local regeneration in perennial species, but vegetative regeneration alone does not establish invasive potential. Fragmentation-assisted establishment is documented for H. moscheutos. (Canada) |
Economic Importance
Economic significance within Hibiscus is concentrated in a relatively small number of cultivated species, particularly ornamental taxa and species historically associated with roselle and kenaf production. Under the current Kew treatment, roselle is treated as Sabdariffa gossypiifolia (historically Hibiscus sabdariffa L.), while kenaf is treated as Sabdariffa cannabina (historically Hibiscus cannabinus L.). These nomenclatural changes are important when interpreting economic literature, much of which continues to use the historical Hibiscus combinations.
Roselle is cultivated for calyces used in beverages and food products, while kenaf is primarily an industrial fibre crop. Ornamental Hibiscus species also have substantial horticultural importance. A comparable genus-wide quantitative market estimate is not established.
| Use Category | Description | Economic Impact |
|---|---|---|
| Food and beverage | Sabdariffa gossypiifolia (historically Hibiscus sabdariffa) is cultivated for calyces used in beverages, herbal teas, jellies and related food products; leaves and other plant parts also have documented local food uses. | Regional and international specialty-botanical trade; the economic importance varies by production system and market. |
| Fibre | Sabdariffa cannabina (historically Hibiscus cannabinus) and other fibre-producing taxa provide bast fibre used for cordage, sacks, yarn, pulp and related materials. | Established fibre-crop significance, particularly for kenaf and related commercial fibre crops; economic scale varies geographically. |
| Ornamental horticulture | Species including Hibiscus rosa-sinensis and Hibiscus syriacus are widely cultivated for flowers, gardens and landscaping. | Broad horticultural significance, but standardized genus-wide market statistics are unavailable. |
| Seeds and coproducts | Selected species provide edible seeds, seed oil, fodder and other coproducts. | Can add value to multipurpose crops, but the economic scale varies substantially among species and regions. |
Economic Assessment
Economic importance is concentrated in three principal areas: food and beverage production associated with roselle, industrial fibre production associated with kenaf and related taxa, and ornamental horticulture.
Assessment: Substantial but highly species- and product-specific; no defensible genus-wide monetary valuation was identified.
The available literature also identifies supply-chain vulnerability in roselle production. Production may be labour-intensive, commercial information can be incompletely tracked, and product quality can be affected by pests, diseases, and post-harvest conditions.
Traditional Uses
Documented traditional uses are strongly species-specific. The following examples retain the identified knowledge system or cultural community rather than treating all Hibiscus uses as a single tradition. Historical scientific names are retained where necessary to maintain traceability to the cited ethnobotanical literature.
| Use Category | Knowledge System | Region or Cultural Group | Practice Summary | Documentation Level | Source |
|---|---|---|---|---|---|
| Food and medicinal use | Indian traditional medicine / Ayurveda-related literature | India | Sabdariffa gossypiifolia (historically Hibiscus sabdariffa L.) leaves, calyces, petals and flowers are documented as food and traditional medicinal materials. | Documented review synthesis | Kumar et al., 2018 |
| Hair and topical use | Tamil traditional healing | Kancheepuram District, Tamil Nadu | Fresh Hibiscus rosa-sinensis leaves are used in a topical hair preparation. | Field ethnobotanical documentation | Ignacimuthu et al., 2006 |
| Women’s health and other medicinal uses | Tribal medicinal knowledge | Tripura, Northeast India | Hibiscus rosa-sinensis roots, leaves and buds are documented in preparations associated with reproductive and other health concerns. | Field ethnobotanical documentation | Roy et al., 2017 |
| Hair and skin-related use | Ethnomedicinal knowledge | Northern Bengal, India | Hibiscus rosa-sinensis is documented for hair-related and other medicinal applications. | Field ethnobotanical documentation | Banerjee et al., 2018 |
| Skin/hair and other uses | Ethnobotanical knowledge | Barpeta District, Assam | Hibiscus rosa-sinensis leaves are documented in a topical preparation for dandruff. | Field ethnobotanical documentation | Nath et al., 2023 |
These records document traditional use, not clinical efficacy. Traditional-use records should therefore remain distinct from the medicinal-evidence hierarchy established elsewhere in the profile.
Traditional Use Summary
Traditional use is concentrated particularly in South Asian knowledge systems, with Hibiscus rosa-sinensis and the taxon currently accepted as Sabdariffa gossypiifolia (historically Hibiscus sabdariffa) repeatedly documented in the cited literature.
The relationship between traditional use and commercialization differs among taxa. Roselle has developed from regional food and beverage use into broader specialty-botanical commerce, whereas many medicinal and cosmetic uses documented for ornamental Hibiscus remain primarily regional or household practices.
Regional Ethnobotanical Context
The ethnobotanical record demonstrates continuity of Hibiscus use across several Indian regions and knowledge communities, but it does not represent a single uniform Indian tradition. Regional surveys from Tamil Nadu, Tripura, Assam, and northern Bengal document different plant parts and applications, indicating localized knowledge transmission.
The available literature is also disproportionately concentrated on India and on a limited number of culturally prominent species. Comparable systematic documentation from many other native-range regions is less developed. Therefore, absence from the surveyed literature should not be interpreted as evidence of absence of traditional use.
Traditional Ecological Knowledge
Documented evidence for specifically ecological knowledge—such as Hibiscus use in agroforestry systems, living fences, ecological indicators, or community resource-management practices—is insufficient at genus level to support a consolidated traditional ecological knowledge (TEK) account.
Ethical Considerations
Community-origin ethnobotanical knowledge is documented in regional surveys, but no specific biopiracy dispute or legally adjudicated intellectual-property conflict involving the genus was identified in the sources reviewed for this turn.
Commercialization of traditionally used species creates an attribution and benefit-sharing context, but a species- or community-specific benefit-sharing arrangement cannot be inferred without documented evidence.
Cultural Significance
Cultural and religious significance is documented for H. rosa-sinensis in Hindu practice. In West Bengal, red hibiscus flowers are documented as offerings to Goddess Kali, and ethnobotanical literature also records use of hibiscus flowers in worship of Durga and Kali. This significance is distinct from the plant’s medicinal, ornamental, or food uses.
The cultural association is therefore particularly well documented in parts of eastern India, although it should not be generalized to all Hibiscus species or all Hindu communities.
Cultivation Summary
Cultivation suitability within the genus is highly heterogeneous. Roselle and kenaf are established annual crop species, while other Hibiscus are cultivated primarily as ornamentals or landscape plants. Biological suitability depends on species-specific temperature, rainfall, photoperiod, reproductive timing, and soil conditions established in earlier turns.
The genus contains both seed-propagated annual crops and perennial ornamental or wild taxa capable of vegetative regeneration. No single cultivation model therefore applies across Hibiscus. Detailed production or propagation procedures are outside this turn.
Pest, Disease and Physiological Burden Summary
The strongest documented production-burden evidence concerns roselle and kenaf.
Roselle is affected by multiple insect pests, including borers, aphids, mealybugs, flea beetles, leaf miners and leafhoppers. Diseases can affect roots, stems, leaves and calyces, with documented consequences for yield and product quality.
In Indian mesta production, major documented burdens include spiral borer, aphid, mealybug, whitefly, root rot and stem rot. Yellow vein mosaic is also documented in H. cannabinus and H. sabdariffa, with whitefly-mediated transmission reported.
These records are species- and production-system-specific and do not constitute a genus-wide pest or disease inventory.
Failure Points and Commercial Risks
Commercial vulnerabilities are concentrated in cultivated species rather than the genus as a whole.
For roselle, quality-sensitive calyx production is vulnerable to pest and disease damage, while labour-intensive harvesting and processing can constrain mechanization. Market information is also comparatively limited because roselle is not consistently tracked as a conventional commodity.
For kenaf and related mesta crops, fibre quality and yield can be affected by insect pests and fungal or viral diseases. Commercial exposure therefore depends on both biological production risks and the particular end-use market.
Conservation Analysis
Conservation cannot be summarized as a single security status for Hibiscus because the genus contains numerous species with very different distributions, population sizes, and threat histories. Cultivation abundance is therefore not evidence of conservation security.
The strongest conservation concern identified at genus level is uneven protection of wild genetic diversity. Some species are widespread and cultivated, whereas narrowly distributed island endemics can be extremely restricted. Hibiscus liliiflorus, for example, has undergone population-level genetic assessment specifically because of its extreme rarity; that study found only two wild individuals remaining at the time of assessment and demonstrated that ex-situ collections did not represent all extant wild genotypes.
Habitat loss is consequently important at the species level, but its severity cannot legitimately be generalized across the genus. Genetic erosion is another conservation dimension: recent work on Hibiscus genetic resources and chloroplast genomes demonstrates substantial interspecific and population-level diversity while also documenting unresolved phylogenetic relationships.
Commercial cultivation has potential conservation value through germplasm maintenance, but cultivated stocks can also represent only a subset of wild genetic diversity. Conservation assessments should therefore distinguish wild population security, genetic representation, and cultivated availability rather than treating them as equivalent.
Conservation Status
| Parameter | Value | Notes | Source |
|---|---|---|---|
| IUCN Red List Category | Not assessed at genus level | IUCN Red List assessments apply to assessed taxa; no genus-level category for Hibiscus was identified. Species-level assessments vary. | IUCN Red List |
| Population Trend | Not established at genus level | Population trends are species-specific; a genus-wide trend cannot be inferred from individual assessments. | IUCN assessment framework |
| Primary Conservation Concern | Species-level habitat and genetic-diversity risk | Particularly important for restricted-range and island-endemic species; severity varies by species. | Species conservation literature |
| Major Conservation Approach | Species-specific in-situ plus genetically representative ex-situ conservation | Genetic assessment of H. liliiflorus demonstrates the importance of retaining representation of wild genotypes. | Mashburn et al., 2023 |
| IUCN URL | No species-specific URL applicable to genus-level target | The target is the genus Hibiscus L.; no genus-specific IUCN assessment page was identified. IUCN’s assessment documentation confirms that assessments are conducted for individual taxa. (IUCN Red List) | IUCN Red List |
| Access Date | 17 September 2026 | IUCN Red List |
Important scope qualification: because the authoritative target is the genus Hibiscus L., the module’s species-level requirement for a species-specific IUCN assessment URL cannot be literally satisfied without changing the established taxonomic target. That is a framework-level rank mismatch, not evidence that Hibiscus is unassessed in every conservation context.
Conservation Risk Factors
| Risk Factor | Severity | Evidence Status |
|---|---|---|
| Habitat loss in restricted-range species | Species-dependent | Verified at selected species level |
| Extremely small wild populations | Potentially severe in individual endemics | Verified for H. liliiflorus |
| Loss of within-species genetic diversity | Species-dependent | Supported; demonstrated conservation relevance in genetic assessments |
| Incomplete representation of wild genotypes in ex-situ collections | Potentially significant for rare taxa | Verified for H. liliiflorus |
| Taxonomic uncertainty and unresolved species boundaries | Indirect conservation risk | Supported by recent phylogenomic work showing complex relationships within Hibiscus and related genera |
Conservation Assessment
The genus should be regarded as conservation-heterogeneous rather than uniformly secure or threatened. Species with broad distributions and substantial cultivation may face different risks from narrowly endemic wild taxa. The strongest direct conservation evidence reviewed here concerns rare species rather than the genus as a whole.
The H. liliiflorus case is particularly informative because it demonstrates that ex-situ abundance does not necessarily preserve the full genetic composition of a wild population. Conservation planning for rare Hibiscus therefore requires population-level information rather than reliance on cultivation status alone.
Research Coverage and Knowledge Gaps
| Research Topic | Coverage Level | Key Gaps | Priority |
|---|---|---|---|
| Taxonomy and phylogeny | Moderate–Strong | intergeneric boundaries; unresolved relationships | High |
| Comparative genomics | Moderate and accelerating | broader taxon sampling; population representation | High |
| Conservation genetics | Selective | wild-population sampling; genetic structure; ex-situ representation | High |
| Population monitoring | Sparse and species-specific | long-term population trends | High |
| Climate vulnerability | Selective | comparative multi-species modelling | Medium–High |
| Reproductive ecology | Moderate for selected species | wild pollination networks; reproductive limitation | Medium |
| Seed biology and regeneration | Moderate but species-biased | comparative persistence and regeneration across rare taxa | Medium |
| Ethnobotanical documentation | Moderate, geographically concentrated | underdocumented native-range knowledge systems | Medium |
Research Landscape
Research on Hibiscus is active and appears to be accelerating in genomics, phytochemistry, applied crop science, and species-specific ecological studies. Recent chloroplast-genome work sampled 36 species and explicitly identifies historical neglect and continuing phylogenetic contention as research issues. Research is geographically concentrated around economically important species and regions with established botanical or agricultural research infrastructure, while rare wild species receive much less sustained investigation except where conservation urgency is high. Funding concentration cannot be quantified reliably from the assembled literature because comparable project-level funding data were not identified. This unevenness means that the apparent strength of evidence for Hibiscus is partly a consequence of research concentration rather than uniform knowledge across the genus.
Priority Knowledge Gaps
The highest-value gap is comparative conservation genetics across wild Hibiscus species. Existing genetic studies demonstrate what can be learned from population-level sampling, but comparable datasets are unavailable for much of the genus. Filling this gap would clarify population structure, unique genetic lineages, and whether ex-situ collections adequately represent wild diversity.
A second priority is integrated taxonomy and phylogeny. Recent plastome research identifies polyphyletic relationships and reticulate or incomplete-lineage-sorting signals among Hibiscus and related genera. Better taxonomic resolution would improve the reliability of distribution, conservation, and ecological records.
A third priority is long-term population monitoring of narrowly distributed species. Individual assessments can establish acute rarity, but repeated demographic observations are needed to distinguish persistent decline from short-term fluctuation.
A fourth priority is comparative climate-vulnerability research. Existing modelling is concentrated in selected species, so it cannot establish a common genus-wide response. Linking climate projections with population genetics, phenology, and reproductive success would provide a stronger basis for identifying species-specific vulnerability.
Finally, native-range ethnobotanical documentation remains uneven. Better documentation would preserve attribution and distinguish genuine knowledge systems from generalized secondary claims.
Interesting Facts
- Hibiscus has historically been taxonomically contentious, with molecular evidence continuing to reshape relationships within the genus and among related genera.
- Recent chloroplast-genome research sampled 36 Hibiscus species and identified candidate molecular markers with potential applications in future population-genetic and breeding research.
- Hibiscus liliiflorus provides an important example of conservation genetics within the genus: a study examined a small number of remaining wild genotypes and found that international ex-situ collections did not contain unique genotypes absent from Rodrigues.
- Hibiscus tiliaceus demonstrates how seed dispersal can contribute to a species’ broad geographic distribution, with water-mediated dispersal associated with its pantropical coastal range.
- The genus combines annual crops, perennial herbs, shrubs, trees, ornamentals, fibre-producing taxa and food plants, making a single genus-wide ecological or economic profile inherently heterogeneous.
Frequently Asked Questions
Taxonomy and Identity
Is Hibiscus L. a species or a genus?
It is a genus in the family Malvaceae. The profile deliberately retains Hibiscus L. as the authoritative genus-level taxonomic target.
Can every species commonly called hibiscus be treated as part of the same biological profile?
No. The genus contains substantial ecological, reproductive, physiological, and taxonomic variation. Species-level findings must therefore remain attached to the relevant species.
Ecology and Reproduction
Do all Hibiscus have the same climate requirements?
No. Documented environmental requirements and climatic associations differ substantially among species, including tropical, subtropical, coastal, wetland, seasonally dry and temperate taxa.
Are Hibiscus flowers dependent on one pollinator?
No. Documented pollination systems vary among species, with bees particularly important in several studied taxa.
Uses and Safety
Are medicinal claims about one Hibiscus species applicable to the whole genus?
No. The strongest medicinal evidence in the profile concerns particular species and preparations, especially Sabdariffa gossypiifolia (historically Hibiscus sabdariffa).
Is cultivated Hibiscus automatically conservation-secure?
No. Cultivated abundance does not establish the security or genetic representativeness of wild populations.
Conclusion
Hibiscus L. is a taxonomically complex and ecologically heterogeneous genus encompassing wild plants, crops, ornamentals, fibre species, food plants, and culturally important taxa. Across the completed profile, the strongest general finding is not a single universal trait but substantial biological diversity: species differ in climate envelopes, reproductive systems, stress responses, habitat associations, uses, and conservation circumstances.
The evidence base is strongest for a relatively small group of economically or culturally prominent species. Important gaps remain in comparative taxonomy, wild-population genetics, long-term demographic monitoring, climate vulnerability, reproductive ecology, and representation of under-studied native-range knowledge systems. Conservation evidence particularly demonstrates why cultivated abundance should not be substituted for wild-population assessment.
Taken together, the profile provides a genus-level framework while preserving species-specific evidence where the biology requires it. The resulting research priorities are therefore comparative rather than based on assuming that one well-studied Hibiscus species represents the entire genus. The profile series covers Adaptations, Phenology, Pollination, and Reproductive Biology; Human Interaction and Applied Cultivation Knowledge; Conservation, Research, and Synthesis.
References
A. Primary Taxonomic Sources
- Linnaeus, C. (1753). Species Plantarum. Stockholm: Laurentius Salvius. Original publication of Hibiscus L.
- International Plant Names Index (IPNI). (2026). Hibiscus L. Nomenclatural record.
https://www.ipni.org/
Accessed 17 September 2026. - Royal Botanic Gardens, Kew. (2026). Plants of the World Online: Hibiscus L. Accepted genus, taxonomy and distribution.
https://powo.science.kew.org/
Accessed 17 September 2026.
B. Peer-Reviewed Literature
- Shi, X., Chen, X., Ma, J., Tang, S., Zhu, Z., Li, F., & Chen, G. (2026). Chloroplast genomes provide new insights into the phylogeny and evolution of the genus Hibiscus L. BMC Plant Biology, 26, 429.
https://doi.org/10.1186/s12870-025-08072-7 Annotation: Comparative plastome study examining phylogenetic relationships, evolutionary history, and molecular resources across Hibiscus and related genera. - Mashburn, B., Jhangeer-Khan, R., Bégué, A., Tatayah, V., Olsen, K. M., & Edwards, C. E. (2023). Genetic assessment improves conservation efforts for the critically endangered oceanic island endemic Hibiscus liliiflorus. Journal of Heredity, 114(3), 259–270.
https://doi.org/10.1093/jhered/esad021. Annotation: Species-specific conservation-genetic evidence concerning wild genotypes and ex-situ representation. - Santiago, L. S., Lau, T. S., Melcher, P. J., Steele, O. C., & Goldstein, G. (2000). Morphological and physiological responses of Hawaiian Hibiscus tiliaceus populations to light and salinity. International Journal of Plant Sciences, 161(1), 99–106.
https://doi.org/10.1086/314236. Annotation: Population-level physiological and ecological differentiation in Hibiscus tiliaceus under contrasting light and salinity conditions. - Takayama, K., Tateishi, Y., Murata, J., & Kajita, T. (2008). Gene flow and population subdivision in a pantropical plant with sea-drifted seeds, Hibiscus tiliaceus and its allied species: Evidence from microsatellite analyses. Molecular Ecology, 17(11), 2730–2742.
https://doi.org/10.1111/j.1365-294X.2008.03799.x Annotation: Population connectivity, genetic subdivision and long-distance dispersal in Hibiscus tiliaceus and allied taxa. - Zhang, L., Jiang, B., Meng, Y., Jia, Y., Xu, Q., & Pan, Y. (2024). The influence of climate change on the distribution of Hibiscus mutabilis in China: MaxEnt model-based prediction. Plants, 13(13), 1744.
https://doi.org/10.3390/plants13131744. Annotation: Species-specific climate-suitability modelling using MaxEnt and bioclimatic variables. - Xu, J., Zhao, Y., Wang, C., Yan, Y., & Wen, Y. (2025). From current to future projections: Modeling habitat suitability changes for Hibiscus syriacus L. in China using MaxEnt under climate change. Frontiers in Plant Science, 16, 1551684.
https://doi.org/10.3389/fpls.2025.1551684 Annotation: Species-specific modelling of current and projected future habitat suitability for Hibiscus syriacus under alternative climate scenarios. - Talukdar, S. (1952). Photoperiodic behaviour of Hibiscus sabdariffa, L.N.P.5. Nature, 170, 458–459.
https://doi.org/10.1038/170458a0 Annotation: Foundational experimental evidence concerning photoperiodic flowering response in roselle. The historical name Hibiscus sabdariffa is retained in the citation because it is the name used in the original publication. - Kudoh, H., Shimamura, R., Takayama, K., & Whigham, D. F. (2006). Consequences of hydrochory in Hibiscus. Plant Species Biology, 21(3), 127–133.
https://doi.org/10.1111/j.1442-1984.2006.00158.x. Annotation: Review of water-mediated seed dispersal and its ecological, demographic, and evolutionary consequences in Hibiscus. - Aluri, J. S. R., Kunuku, V. R., Chappidi, P. R., & Kammarchedu, B. J. P. (2020). Pollination ecology of Hibiscus tiliaceus L. (Malvaceae), an evergreen tree species valuable in coastal and inland eco-restoration. Transylvanian Review of Systematical and Ecological Research, 22(2), 47–56.
https://doi.org/10.2478/trser-2020-0010 Annotation: Species-specific pollination, reproductive ecology, flowering and regeneration evidence for Hibiscus tiliaceus. - Mahunu, G. K., Apaliya, M. T., & Osei-Kwarteng, M. (2021). Effect of pests and diseases on Hibiscus sabdariffa quality. In A. A. Mariod, H. E. Tahir, & G. K. Mahunu (Eds.), Roselle (Hibiscus sabdariffa): Chemistry, Production, Products, and Utilization (pp. 33–46). Academic Press.
https://doi.org/10.1016/B978-0-12-822100-6.00004-5. Annotation: Production-related pest and disease burden affecting roselle quality. The historical name Hibiscus sabdariffa is retained because it forms part of the published title of the source. - Abat, J. K., Kumar, S., & Mohanty, A. (2017). Ethnomedicinal, phytochemical and ethnopharmacological aspects of four medicinal plants of Malvaceae used in Indian traditional medicines: A review. Medicines, 4(4), 75.
https://doi.org/10.3390/medicines4040075 Annotation: Review of traditional use, phytochemistry, and ethnopharmacological evidence concerning four Malvaceae plants, including Hibiscus sabdariffa. The historical name is retained because it is the name used in the source. - Muthu, C., Ayyanar, M., Raja, N., & Ignacimuthu, S. (2006). Medicinal plants used by traditional healers in Kancheepuram District of Tamil Nadu, India. Journal of Ethnobiology and Ethnomedicine, 2, 43.
https://doi.org/10.1186/1746-4269-2-43 Annotation: Regional ethnobotanical evidence documenting medicinal plant use by traditional healers in Kancheepuram District, including evidence relevant to Hibiscus rosa-sinensis.
C. Monographs, Books and Technical Reports
- Utteridge, T. M. A., & Jennings, L. V. S. (Eds.). (2022). Trees of New Guinea. Kew Publishing. Annotation: Regional botanical reference covering woody genera of New Guinea, including distribution, ecology, taxonomy, and diagnostic information relevant to Hibiscus.
- Flora of Tropical East Africa. Regional taxonomic and distribution treatments relevant to African Hibiscus.
- Flora Zambesiaca. Regional taxonomic and distribution treatments relevant to African Hibiscus.
- Allen, J. A. (2002). Hibiscus tiliaceus L. In J. Vozzo (Ed.), Tropical Tree Seed Manual: Part II, Species Descriptions. Agriculture Handbook 712, pp. 508–510. U.S. Department of Agriculture, Forest Service. Annotation: Species-specific information on distribution, seed characteristics, and water-mediated dispersal of Hibiscus tiliaceus.
D. Databases and Online Resources
- Royal Botanic Gardens, Kew. (2026). Plants of the World Online (POWO): Hibiscus L.
https://powo.science.kew.org/
Accessed 17 September 2026. - International Plant Names Index (IPNI). (2026). Hibiscus L.
https://www.ipni.org/
Accessed 17 September 2026. - International Union for Conservation of Nature. (2026). IUCN Red List assessment process and supporting information.
https://nrl.iucnredlist.org/assessment/process
Accessed 17 September 2026. - World Flora Online Consortium. World Flora Online.
https://www.worldfloraonline.org/
Accessed 17 September 2026.
E. Grey Literature
- U.S. Forest Service. Fire Effects Information System: Hibiscus moscheutos. Species information concerning phenology, regeneration, seed biology, and reproductive ecology.
- Government of Canada / Committee on the Status of Endangered Wildlife in Canada (COSEWIC). Swamp Rose-mallow (Hibiscus moscheutos): Biology and conservation information.
- Food and Agriculture Organization of the United Nations (FAO). EcoCrop: Hibiscus sabdariffa. Crop and climatic information. The historical name is retained where it represents the database’s source terminology.
- American Society for the Prevention of Cruelty to Animals (ASPCA). Toxic and Non-Toxic Plants: Hibiscus. Species-specific companion-animal safety information.